 +1 credit
| Version | Summary | Created by | Modification | Content Size | Created at | Operation |
|---|---|---|---|---|---|---|
| 1 | Vitalii Ivchuk | -- | 1970 | 2026-10-27 18:20:32 | | | |
| 2 | Catherine Yang | Meta information modification | 1970 | 2026-10-28 02:43:29 | | |
Video Upload Options
Glycosylation in Immune Regulation and Inflammatory Diseases
EditThis entry explores the multifaceted roles of protein and RNA glycosylation in modulating innate and adaptive immunity, highlighting its impact on inflammasome activation and inflammatory disease pathogenesis, and discussing emerging glycan-targeted therapies and diagnostic tools.
1. Introduction
Glycosylation is a fundamental and ubiquitous post-translational modification that involves the enzymatic attachment of carbohydrate structures (glycans) to proteins, lipids, and, most recently discovered, RNAs. It plays a critical role in modulating protein stability, folding, and cellular communication. In recent years, the intricate relationship between glycosylation and the immune system has garnered significant attention. Glycans are essential for the proper function of immune receptors, the regulation of immune cell trafficking, and the fine-tuning of both innate and adaptive immune responses. This review synthesizes current knowledge on the molecular mechanisms by which glycosylation governs immune regulation, with a particular focus on inflammasome activation.
Glycosylation is one of the most common and complex post-translational modifications in biological systems. It involves the covalent attachment of glycans to proteins or lipids, profoundly influencing their structure, stability, localization, and function [1]. It is estimated that over 50% of human proteins are glycosylated, and the majority of cell surface and secreted proteins carry glycan modifications [2]. The glycosylation machinery operates primarily within the endoplasmic reticulum (ER) and the Golgi apparatus, utilizing a vast array of glycosyltransferases and glycosidases. The resulting glycan structures are highly diverse, including N-linked glycans, O-linked glycans, and more specialized forms like C-mannosylation and glycosaminoglycan (GAG) attachment [3][4].
The immune system is particularly reliant on glycosylation. Almost all immune cell surface receptors, cytokines, and antibodies are glycoproteins. Glycans play indispensable roles in immune cell development, activation, and migration, acting as crucial mediators of cell-cell interactions and signal transduction [2]. The "glycocalyx," a dense layer of glycans on the cell surface, dictates the initial interactions between immune cells and their microenvironment. Furthermore, the discovery of glycoRNAs – small RNAs modified with N-glycans – has expanded the paradigm of glycosylation beyond proteins and lipids, suggesting a novel layer of immune regulation [5][6]. The 21st century has seen a breakthrough in glycobiology, driven by advanced analytical techniques and a deeper understanding of complex diseases [7]. This review aims to provide a comprehensive overview of how glycosylation shapes immune responses, focusing on its role in inflammasome activation, its dysregulation in inflammatory diseases and cancer, and its potential as a therapeutic target (Figure 1) [8].
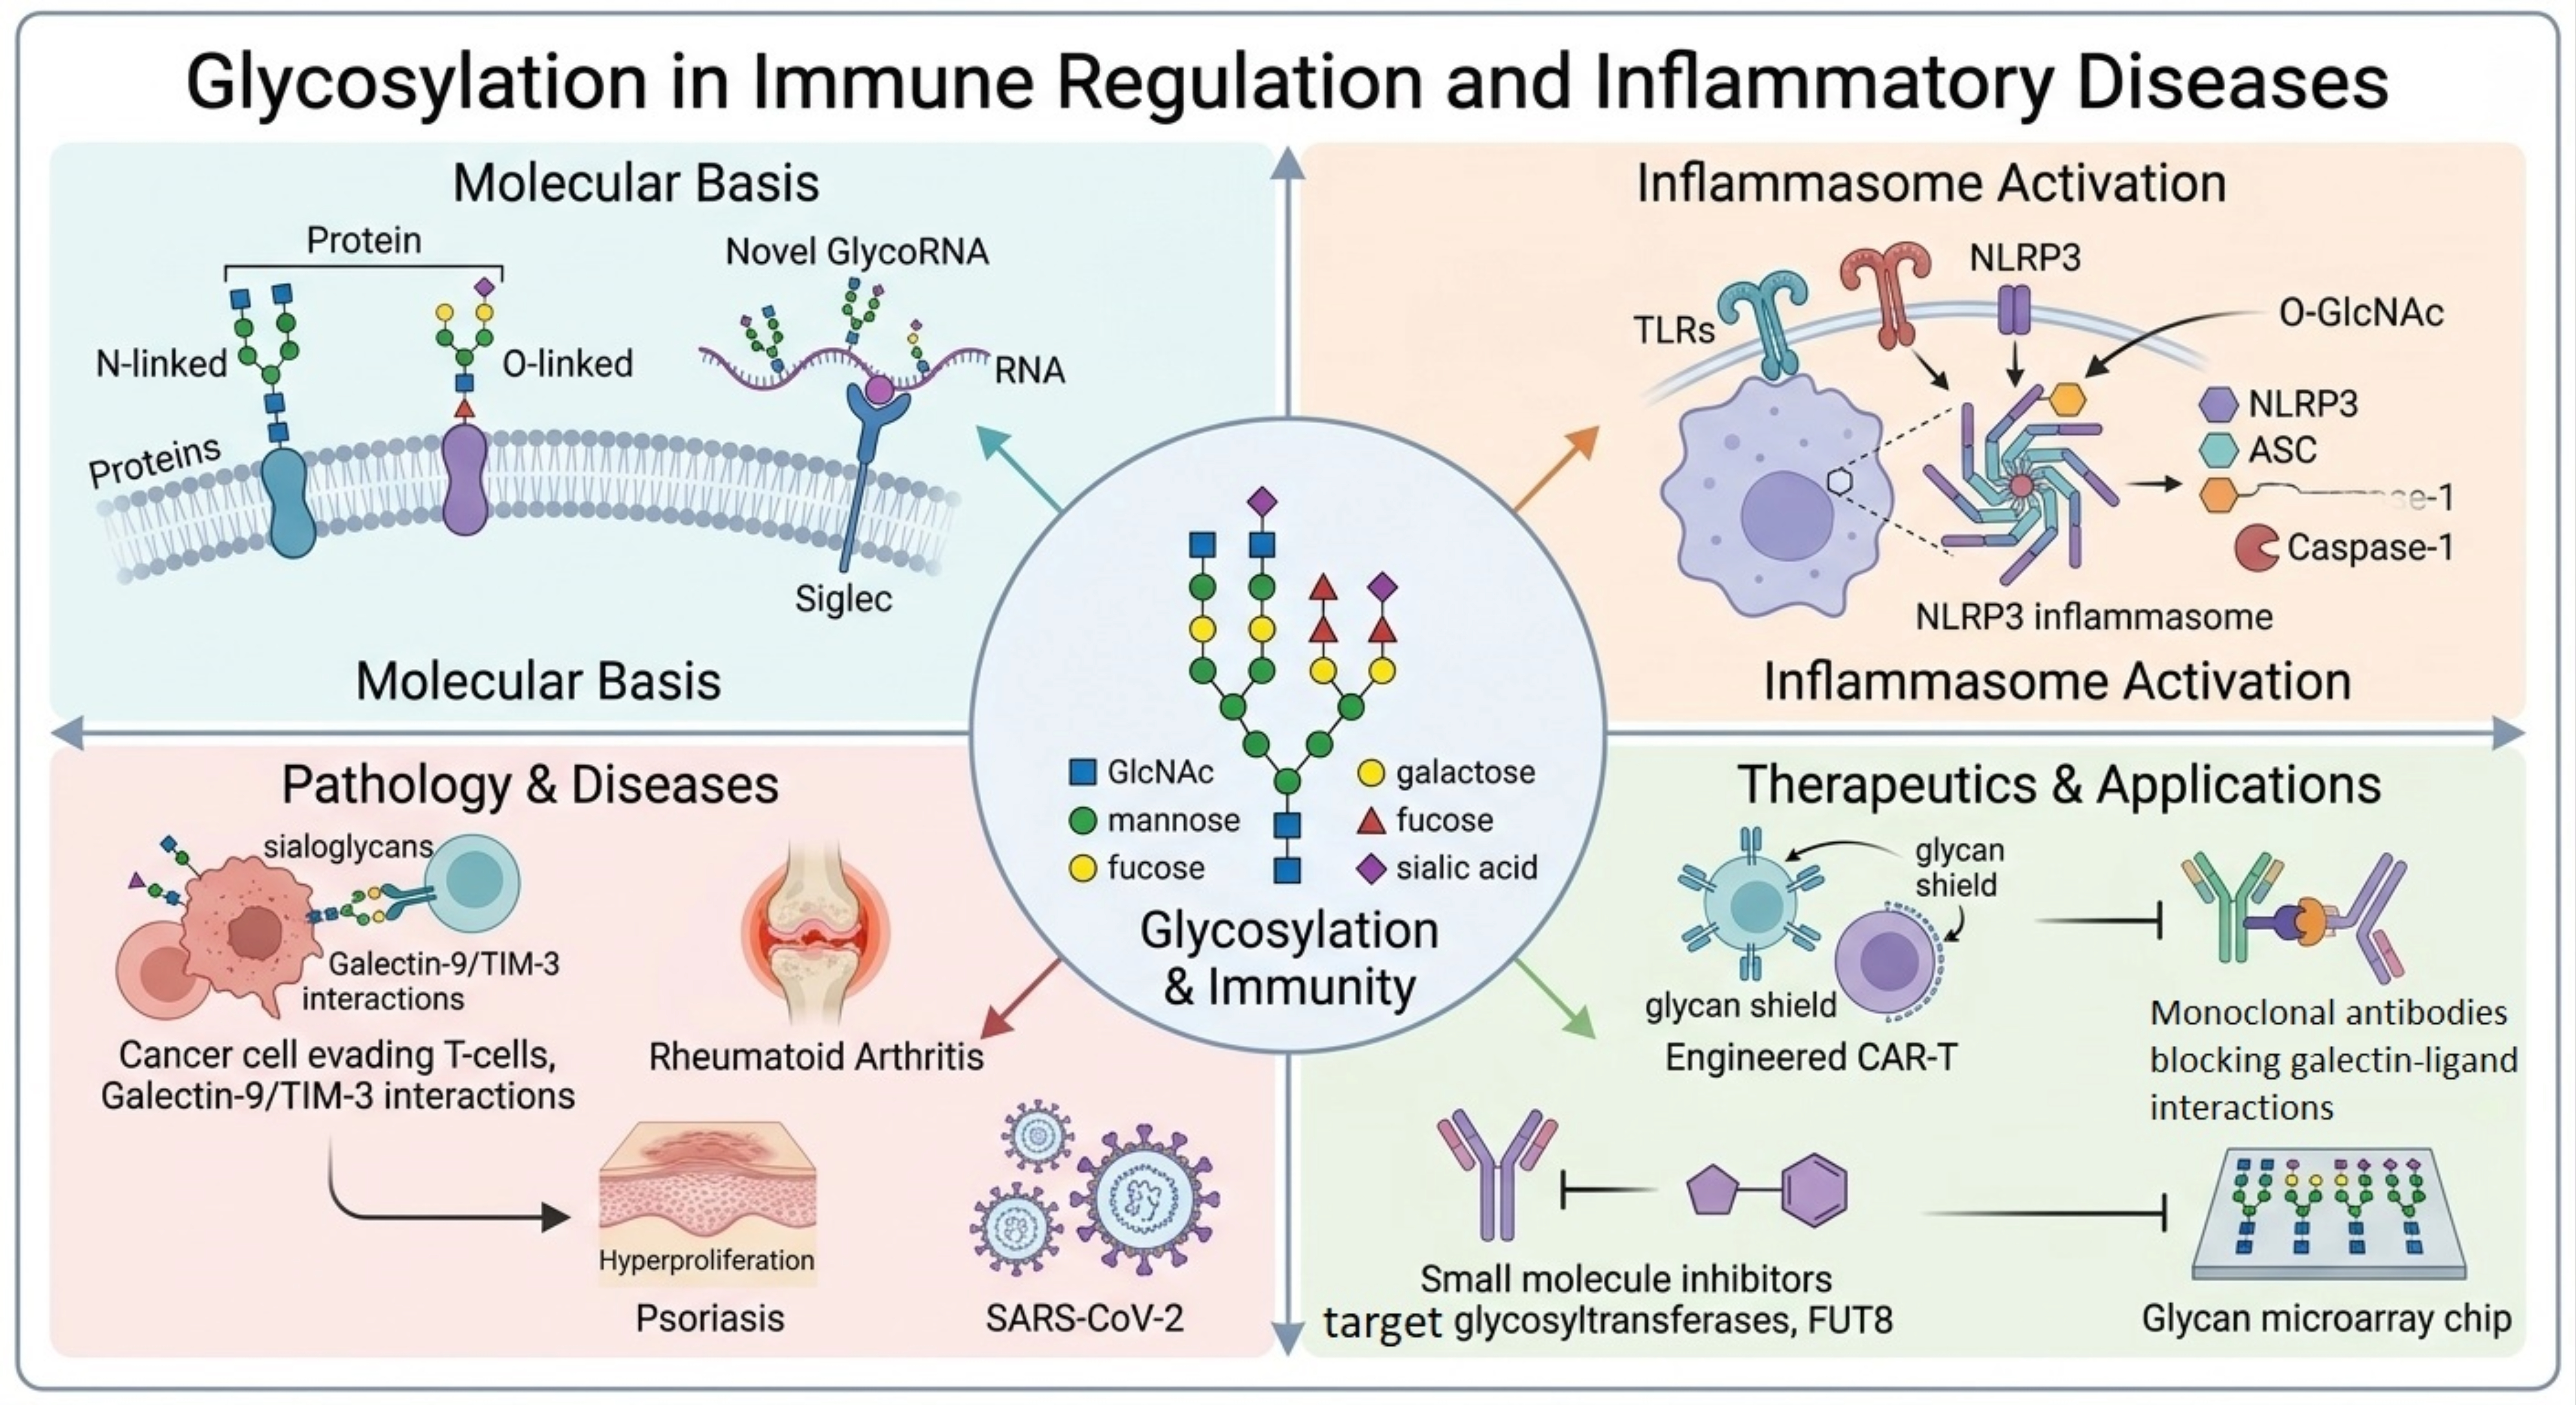
Figure 1. Comprehensive overview of glycosylation in immune regulation and inflammatory diseases. The central hub illustrates the fundamental role of the glycan code, comprising specific monosaccharide building blocks (GlcNAc – blue square, mannose – green circle, fucose – red triangle, galactose – yellow circle, sialic acid – purple diamond). The surrounding four quadrants detail the major thematic areas of this review: (1) Molecular Basis: the interaction of N-linked glycans, O-linked glycans, and emerging glycoRNAs displayed on cell surfaces with immune receptors (such as Siglecs); (2) Inflammasome Activation: glycosylation-dependent regulation of Toll-like receptors (TLRs) and the activation of the NLRP3 inflammasome via O-GlcNAcylation of its components, facilitating complex assembly (ASC, Caspase-1) and pyroptosis; (3) Disease Pathology: aberrant glycosylation driving cancer progression (tumor immune evasion via sialoglycans engaging TIM-3/Galectin-9 checkpoints), pro-inflammatory glycan signatures in rheumatoid arthritis, keratinocyte hyperproliferation in psoriasis, and host glycan exploitation by SARS-CoV-2; (4) Therapeutic Applications: immune cell glycoengineering (constructing protective glycan shields on CAR-T cells), monoclonal antibodies targeting lectin immune checkpoints, small molecule inhibitors of glycosyltransferases (e.g., FUT8), and high-throughput glycan microarray chips for biomarker discovery and diagnostics. Image created using Gemini tool (Google, 2026) based on the directions provided by the author to illustrate this concept. The final image was curated and verified for technical accuracy by the author.
2. The Glycobiology of Immune Recognition
The immune system relies on a sophisticated network of glycan-binding proteins, or lectins, to interpret the glycan code displayed on cells and pathogens. These interactions are fundamental to distinguishing self from non-self and initiating appropriate immune responses. Key lectin families involved in immunity include Siglecs (sialic acid-binding immunoglobulin-like lectins), galectins, and C-type lectin receptors (CLRs) [2]. Tandem-repeat lectins, which contain multiple carbohydrate recognition domains (CRDs) in a single polypeptide chain, are also crucial for multivalent interactions and high-avidity binding in immune recognition [9]. Furthermore, unique carbohydrate modifications such as N-glycolylated sugars, which are non-human sialic acid variants often incorporated through diet, can act as xeno-autoantigens and trigger inflammatory responses (xenosialitis) [10].
Siglecs are predominantly expressed on immune cells and typically contain immunoreceptor tyrosine-based inhibitory motifs (ITIMs) that transmit inhibitory signals. For instance, the engagement of Siglecs by sialylated glycans – which are often upregulated on tumor cells – can suppress immune activation, facilitating immune evasion [2]. Galectins, characterized by their affinity for β-galactoside-containing glycans, are emerging as critical regulators of immunity. A prominent example is Galectin-9 (Gal-9), which contains two distinct CRDs connected by a linker peptide, allowing it to bind a diverse repertoire of glycoprotein receptors [11]. Gal-9 is a pivotal mediator in the tumor microenvironment, where it interacts with immune checkpoint receptors like TIM-3 and PD-1 on T cells, inducing T cell exhaustion and apoptosis [11].
To study these complex interactions, glycan microarrays have emerged as powerful high-throughput tools. These arrays allow for the interrogation of glycan-binding specificities of lectins and antibodies, revealing unique glycan recognition profiles that underpin immune functions [12]. Additionally, structural biology approaches, such as the analysis of sulfotransferase structures, have provided critical insights into how specific sulfation patterns on glycans dictate their interactions with immune receptors and signaling molecules [13].
3. Glycosylation as a Master Regulator of Inflammasome Activation
Inflammasomes are multiprotein complexes that form a critical component of the innate immune response, sensing pathogenic threats and endogenous danger signals. The most extensively studied is the NLRP3 inflammasome, which requires two signals for activation: a priming signal (often via Toll-like receptors, TLRs) and an activation signal. Emerging evidence indicates that glycosylation regulates both stages [14].
3.1. Glycans in Inflammasome Priming
The priming signal for NLRP3 is intricately linked to the glycosylation of TLRs and their co-receptors. For example, the proper N-linked glycosylation of MD-2 and TLR4 is essential for their cell surface transport and functional integrity in recognizing lipopolysaccharides (LPS) [14]. Similarly, CD14, a co-receptor for TLR4, requires N-linked glycosylation for proper folding, secretion, and interaction with ligands [14]. Furthermore, the fucosylation of these receptors is crucial for LPS-induced inflammation and internalization [14]. These findings highlight that structural glycan modifications are prerequisites for the initiation of inflammatory signaling.
3.2. Glycosylation of Inflammasome Components
Beyond the priming stage, the activation of the NLRP3 inflammasome is directly modulated by the O-GlcNAcylation of its components. O-GlcNAc transferase (OGT) catalyzes the addition of N-acetylglucosamine to serine or threonine residues. Research has demonstrated that O-GlcNAcylation of NLRP3 at Thr542 promotes its activation and subsequent pyroptosis [14]. Similarly, the O-GlcNAcylation of NEK7 and TXNIP enhances their interaction with NLRP3, facilitating inflammasome assembly under high-glucose conditions [14]. Additionally, the effector molecules of pyroptosis, such as GSDMD and GSDME, are also subject to O-GlcNAcylation, which can either inhibit or promote their pore-forming activity [14].
4. Glycan Dysregulation in Diseases: Cancer, Autoimmunity, and Infection
Aberrant glycosylation is a hallmark of several chronic inflammatory, autoimmune, and neoplastic diseases, often contributing to disease severity and progression.
4.1. Cancer
In cancer, altered glycosylation supports tumor progression, metastasis, and immune evasion. In prostate cancer, for instance, increased branching of complex N-glycans, altered sialylation, and changes in fucosylation are common [15]. Specifically, the upregulation of α-(1,6)-fucosyltransferase 8 (FUT8) leads to core fucosylation of malignant N-glycans, which promotes tumor growth [16]. Fucosylation is also heavily implicated in urological cancers, where specific fucosyltransferases mediate tumor aggressiveness and serve as potential biomarkers [17]. Glycosylation also plays a crucial role in shaping the tumor immune microenvironment, with sialoglycans engaging inhibitory Siglec receptors on immune cells to suppress antitumor immunity [2]. The role of Galectin-9 as a glyco-immune checkpoint is also being actively explored as a target for cancer therapy [11].
4.2. Autoimmune and Inflammatory Diseases
In rheumatic diseases such as rheumatoid arthritis (RA), there is a well-documented shift in the glycosylation profile of Immunoglobulin G (IgG). Autoantigen-specific IgG in RA patients exhibits a distinct N-glycosylation signature characterized by a lack of terminal sialylation and galactosylation (G0F glycans), which correlates with disease activity and a pro-inflammatory state [18]. Glycosylation also plays a critical role in osteoclast differentiation and bone resorption, key processes in RA and osteoporosis [19]. Furthermore, glucocorticoids, a mainstay treatment for RA, have been shown to affect the expression of proteoglycans and glycosaminoglycans, altering the extracellular matrix and disease trajectory [20]. In psoriasis, elevated expression of FUT8 increases core fucosylation of the epidermal growth factor receptor (EGFR), promoting keratinocyte proliferation [21].
4.3. Infectious Diseases
Pathogens have evolved sophisticated strategies to exploit host glycosylation. Viruses such as SARS-CoV-2 utilize host sialylated receptors for cellular entry and incorporate host-derived glycan structures to form a "glycan shield" [22]. Microbial pathogens also exploit glycosphingolipids on host cell membranes to invade, dupe, or kill host cells, utilizing specific lectins for recognition [23]. The attachment of uropathogenic E. coli (UPEC) to the urothelium is mediated by the FimH adhesin binding to mannose-containing host glycoproteins. Conversely, host glycans on the urothelial surface and on secreted glycoproteins like Tamm-Horsfall protein prevent or limit infection by inhibiting UPEC adhesion [24]. Similar glycan-dependent interactions are pivotal in rotavirus and norovirus infections, where host histo-blood group antigens serve as key receptors [25].
5. Emerging Concepts and Technological Advances
Recent technological advances are driving the field forward. The discovery of glycoRNAs – small RNAs modified with N-glycans and displayed on the cell surface – has expanded the paradigm of glycosylation. These glycoRNAs interact with glycan-binding proteins like Siglecs, playing roles in immune recognition and cell-cell communication [5][6]. Furthermore, the application of single-cell sequencing and spatial transcriptomics is enabling researchers to map the expression of GAG-associated enzymes and resolve cell-type specific glycan signatures in complex tissues [26]. Recent studies have even mapped the spatial distribution of N- and O-glycans in the mammalian brain, revealing unique tissue-specific expression patterns [27]. Advanced mass spectrometry and structural biology techniques (cryo-EM, NMR) are also providing unprecedented insights into the structure-function relationships of glycans and their receptors [28][29].
6. Therapeutic Implications and Translational Potential
The profound influence of glycosylation on immunity has spurred the development of novel glyco-based therapeutic strategies.
6.1. Glycoengineering of Immune Cells
Manipulating the glycosylation machinery of immune cells is a promising avenue for enhancing cell-based therapies. For instance, knocking out SPPL3, a negative regulator of glycosylation, creates a "glycan shield" on CAR-T cells that mitigates allogeneic rejection [2]. Chemoenzymatic engineering of natural killer (NK) cells with synthetic glycan ligands can also equip them with high-affinity targeting capabilities for specific tumor receptors [2].
6.2. Targeting Glycan-Lectin Interactions
Blocking the immunosuppressive interactions mediated by lectins is a key strategy. Monoclonal antibodies targeting Gal-9 (e.g., Lyt-200) or its receptors (TIM-3) are undergoing clinical trials for solid tumors and hematological malignancies [11]. Furthermore, inhibiting the glycosylation of immune checkpoint proteins, such as the core fucosylation of PD-1, can enhance anti-tumor immunity [2]. Small molecule inhibitors that target specific glycosyltransferases (like FUT8) or glycosidases are also being explored [16]. Beyond direct inhibition, glycomaterials with engineered selectivity and affinity are being developed to precisely target specific lectin interactions [30].
6.3. Novel Glyco-based Biomaterials and Therapeutics
Glycosylation is also central to tissue regeneration and reproductive biology. Glycosaminoglycans (GAGs) are being engineered as biomaterials for tissue repair, utilizing their inherent biocompatibility and bioactivity [31]. In reproductive glycobiology, targeting specific glycan-lectin interactions is being explored to address complications like implantation failure and preeclampsia [32]. Additionally, the chemical synthesis of glycopeptides and glycopeptide conjugates is enabling the development of highly specific vaccines and immunotherapeutics, bypassing the heterogeneity of natural glycoproteins [33].
7. Conclusions
Glycosylation is a fundamental process that intricately regulates immune function and inflammation. From the initial recognition of pathogens by lectins to the fine-tuning of inflammasome activation and the regulation of immune checkpoints, glycans are ubiquitous and indispensable. The dysregulation of these pathways is a key driver in the pathogenesis of inflammatory diseases, autoimmunity, and cancer. With the discovery of new glycan structures, such as glycoRNAs, and the development of sophisticated glycoengineering technologies, the field is poised for significant breakthroughs. Targeting glycosylation pathways and glycan-lectin interactions offers a promising frontier for the development of next-generation precision immunotherapies and anti-inflammatory treatments.
References
- Katrine T. Schjoldager; Yoshiki Narimatsu; Hiren J. Joshi; Henrik Clausen; Global view of human protein glycosylation pathways and functions. Nat. Rev. Mol. Cell Biol. 2020, 21, 729-749. [CrossRef]
- Shengwen Ding; Han Wang; Zhaoxin Han; Senlian Hong; Immunomodulation by glycosylation: bridging glycobiology to adaptive immunity and therapeutic innovation. Front. Immunol. 2026, 17, 1729274. [CrossRef]
- Tiago Oliveira; Morten Thaysen-Andersen; Nicolle H. Packer; Daniel Kolarich; The Hitchhiker's guide to glycoproteomics. Biochem. Soc. Trans. 2021, 49, 1643-1662. [CrossRef]
- Courtney J. Mycroft-West; Miron A. Leanca; Liang Wu; Structural glycobiology – from enzymes to organelles. Biochem. Soc. Trans. 2025, 53, 83-100. [CrossRef]
- Ryan A. Flynn; Kayvon Pedram; Stacy A. Malaker; Pedro J. Batista; Benjamin A.H. Smith; Alex G. Johnson; Benson M. George; Karim Majzoub; Peter W. Villalta; Jan E. Carette; Carolyn R. Bertozzi; Small RNAs are modified with N-glycans and displayed on the surface of living cells. Cell 2021, 184, 3109-3124.e22. [CrossRef]
- Nicole Montag; Pavlos Gousis; Jürgen Wittmann; The emerging role of GlycoRNAs in immune regulation and recognition. Immunol. Lett. 2025, 276, 107048. [CrossRef]
- Gehendra Mahara; Cuihong Tian; Xiaojia Xu; Jinxiu Zhu; Breakthrough of glycobiology in the 21st century. Front. Immunol. 2023, 13, 1071360. [CrossRef]
- Vitalii Ivchuk. Glycosylation as a Universal Regulator of Pathogenesis and Therapeutic Target in Multifactorial Human Diseases; MDPI AG: Basel, Switzerland, 2026. [CrossRef]
- Francisco H Olvera-Lucio; Héctor Riveros-Rosas; Adrián Quintero-Martínez; Alejandra Hernández-Santoyo; Tandem-repeat lectins: structural and functional insights. Glycobiology 2024, 34, cwae041. [CrossRef]
- Adeola E Awofiranye; Chirag Dhar; Peng He; Ajit Varki; Mattheos A G Koffas; Robert J Linhardt; N-glycolylated carbohydrates in nature. Glycobiology 2022, 32, 921-932. [CrossRef]
- Anastasia Iris Karkempetzaki; Tobias Schatton; Steven R. Barthel; Galectin-9—An Emerging Glyco-Immune Checkpoint Target for Cancer Therapy. Int. J. Mol. Sci. 2025, 26, 7998. [CrossRef]
- Jamie Heimburg-Molinaro; Akul Y. Mehta; Catherine A. Tilton; Richard D. Cummings; Insights Into Glycobiology and the Protein-Glycan Interactome Using Glycan Microarray Technologies. Mol. Cell. Proteom. 2024, 23, 100844. [CrossRef]
- Lars C. Pedersen; MyeongJin Yi; Lee G. Pedersen; Andrea M. Kaminski; From Steroid and Drug Metabolism to Glycobiology, Using Sulfotransferase Structures to Understand and Tailor Function. Drug Metab. Dispos. 2022, 50, 1027-1041. [CrossRef]
- Hongliang Zhang; Tengchuan Jin; Mengzhou Xue; Songquan Wu; Chunfu Zheng; When glycobiology meets inflammasome activation: Insights and implications. J. Adv. Res. 2025, 79, 833-846. [CrossRef]
- William Butler; Jiaoti Huang; Glycosylation Changes in Prostate Cancer Progression. Front. Oncol. 2021, 11, 809170. [CrossRef]
- Kirsty Hodgson; Margarita Orozco-Moreno; Ziqian Peng; Libby Blencoe; Molly J. Sharp; Erin Smith; Grace Grimsley; David J. Elliott; Richard Beatson; Richard R. Drake; Jennifer Munkley; The glycobiology of prostate cancer: an update. Oncogene 2026, 45, 2655-2670. [CrossRef]
- Kazutoshi Fujita; Koji Hatano; Mamoru Hashimoto; Eisuke Tomiyama; Eiji Miyoshi; Norio Nonomura; Hirotsugu Uemura; Fucosylation in Urological Cancers. Int. J. Mol. Sci. 2021, 22, 13333. [CrossRef]
- Theresa Kissel; René E. M. Toes; Thomas W. J. Huizinga; Manfred Wuhrer; Glycobiology of rheumatic diseases. Nat. Rev. Rheumatol. 2022, 19, 28-43. [CrossRef]
- Shufa Yang; Ziyi He; Tuo Wu; Shunlei Wang; Hui Dai; Glycobiology in osteoclast differentiation and function. Bone Res. 2023, 11, 1-14. [CrossRef]
- Anastasia V. Strokotova; Elvira V. Grigorieva; Glucocorticoid Effects on Proteoglycans and Glycosaminoglycans. Int. J. Mol. Sci. 2022, 23, 15678. [CrossRef]
- Yinuo Yang; Xin Zhou; Wenhui Wang; Hui Dai; Glycobiology of psoriasis: A review. J. Autoimmun. 2025, 151, 103361. [CrossRef]
- Yanqiu Gong; Suideng Qin; Lunzhi Dai; Zhixin Tian; The glycosylation in SARS-CoV-2 and its receptor ACE2. Signal Transduct. Target. Ther. 2021, 6, 1-24. [CrossRef]
- Anna Bereznicka; Krzysztof Mikolajczyk; Marcin Czerwinski; Radoslaw Kaczmarek; Microbial lectome versus host glycolipidome: How pathogens exploit glycosphingolipids to invade, dupe or kill. Front. Microbiol. 2022, 13, 958653. [CrossRef]
- Federico Lupo; Molly A. Ingersoll; Miguel A. Pineda; The glycobiology of uropathogenic E. coli infection: the sweet and bitter role of sugars in urinary tract immunity. Immunology 2021, 164, 3-14. [CrossRef]
- Nazaret Peña-Gil; Cristina Santiso-Bellón; Roberto Gozalbo-Rovira; Javier Buesa; Vicente Monedero; Jesús Rodríguez-Díaz; The Role of Host Glycobiology and Gut Microbiota in Rotavirus and Norovirus Infection, an Update. Int. J. Mol. Sci. 2021, 22, 13473. [CrossRef]
- Lalhaba Oinam; Hiroaki Tateno; Glycan Profiling by Sequencing to Uncover Multicellular Communication: Launching Glycobiology in Single Cells and Microbiomes. Front. Cell Dev. Biol. 2022, 10, 919168. [CrossRef]
- Maxence Noel; Yumi M Zürcher; Ea K C Tulin; Richard D Cummings; The Importance of N- and O-Glycosylation of Brain Cell Surface Glycoproteins. Glycobiology 2025, 35, cwaf054. [CrossRef]
- Ignacio Sanz-Martinez; Sandra Pereira; Pedro Merino; Francisco Corzana; Ramon Hurtado-Guerrero; Molecular Recognition of GalNAc in Mucin-Type O-Glycosylation. Acc. Chem. Res. 2023, 56, 548-560. [CrossRef]
- Melissa Koff; Pedro Monagas-Valentin; Boris Novikov; Ishita Chandel; Vladislav Panin; Protein O-mannosylation: one sugar, several pathways, many functions. Glycobiology 2023, 33, 911-926. [CrossRef]
- Sarah-Jane Richards; Matthew I. Gibson; Toward Glycomaterials with Selectivity as Well as Affinity. JACS Au 2021, 1, 2089-2099. [CrossRef]
- Alvile Kasarinaite; Junhan Ou; Kailin Chen; Dayang Peng; Wendi Jia; Chenyang Ding; Wenwen Huang; David C. Hay; Yishan Chen; Glycosaminoglycans in tissue regeneration: Insights into glycobiology and their biomedical application. Bioact. Mater. 2026, 60, 320-337. [CrossRef]
- Jiangming Zhong; Jianlin Li; Graham J Burton; Hannu Koistinen; Ka Wang Cheung; Ernest H Y Ng; Yuanqing Yao; William S B Yeung; Cheuk-Lun Lee; Philip C N Chiu; The functional roles of protein glycosylation in human maternal–fetal crosstalk. Hum. Reprod. Update 2023, 30, 81-108. [CrossRef]
- Ward Doelman; Sander I. van Kasteren; Synthesis of glycopeptides and glycopeptide conjugates. Org. Biomol. Chem. 2022, 20, 6487-6507. [CrossRef]